How Claude designed protein binders against scorpion neurotoxins
Published
Team
Topics
Summary: As part of our work experimenting with how Claude can help accelerate drug discovery, we asked an internal research model to design minibinders (small proteins that attach tightly to a target) against scorpion neurotoxins. Claude worked from our prompt and four follow-ups, which we developed in collaboration with the financial investment research firm Citrini Research. Teams at Adaptyv Bio and Twist Bioscience experimentally tested 211 designs for binding. Of these, 17 met our criteria. We’re releasing all 211 designs and their data as a resource for the field.
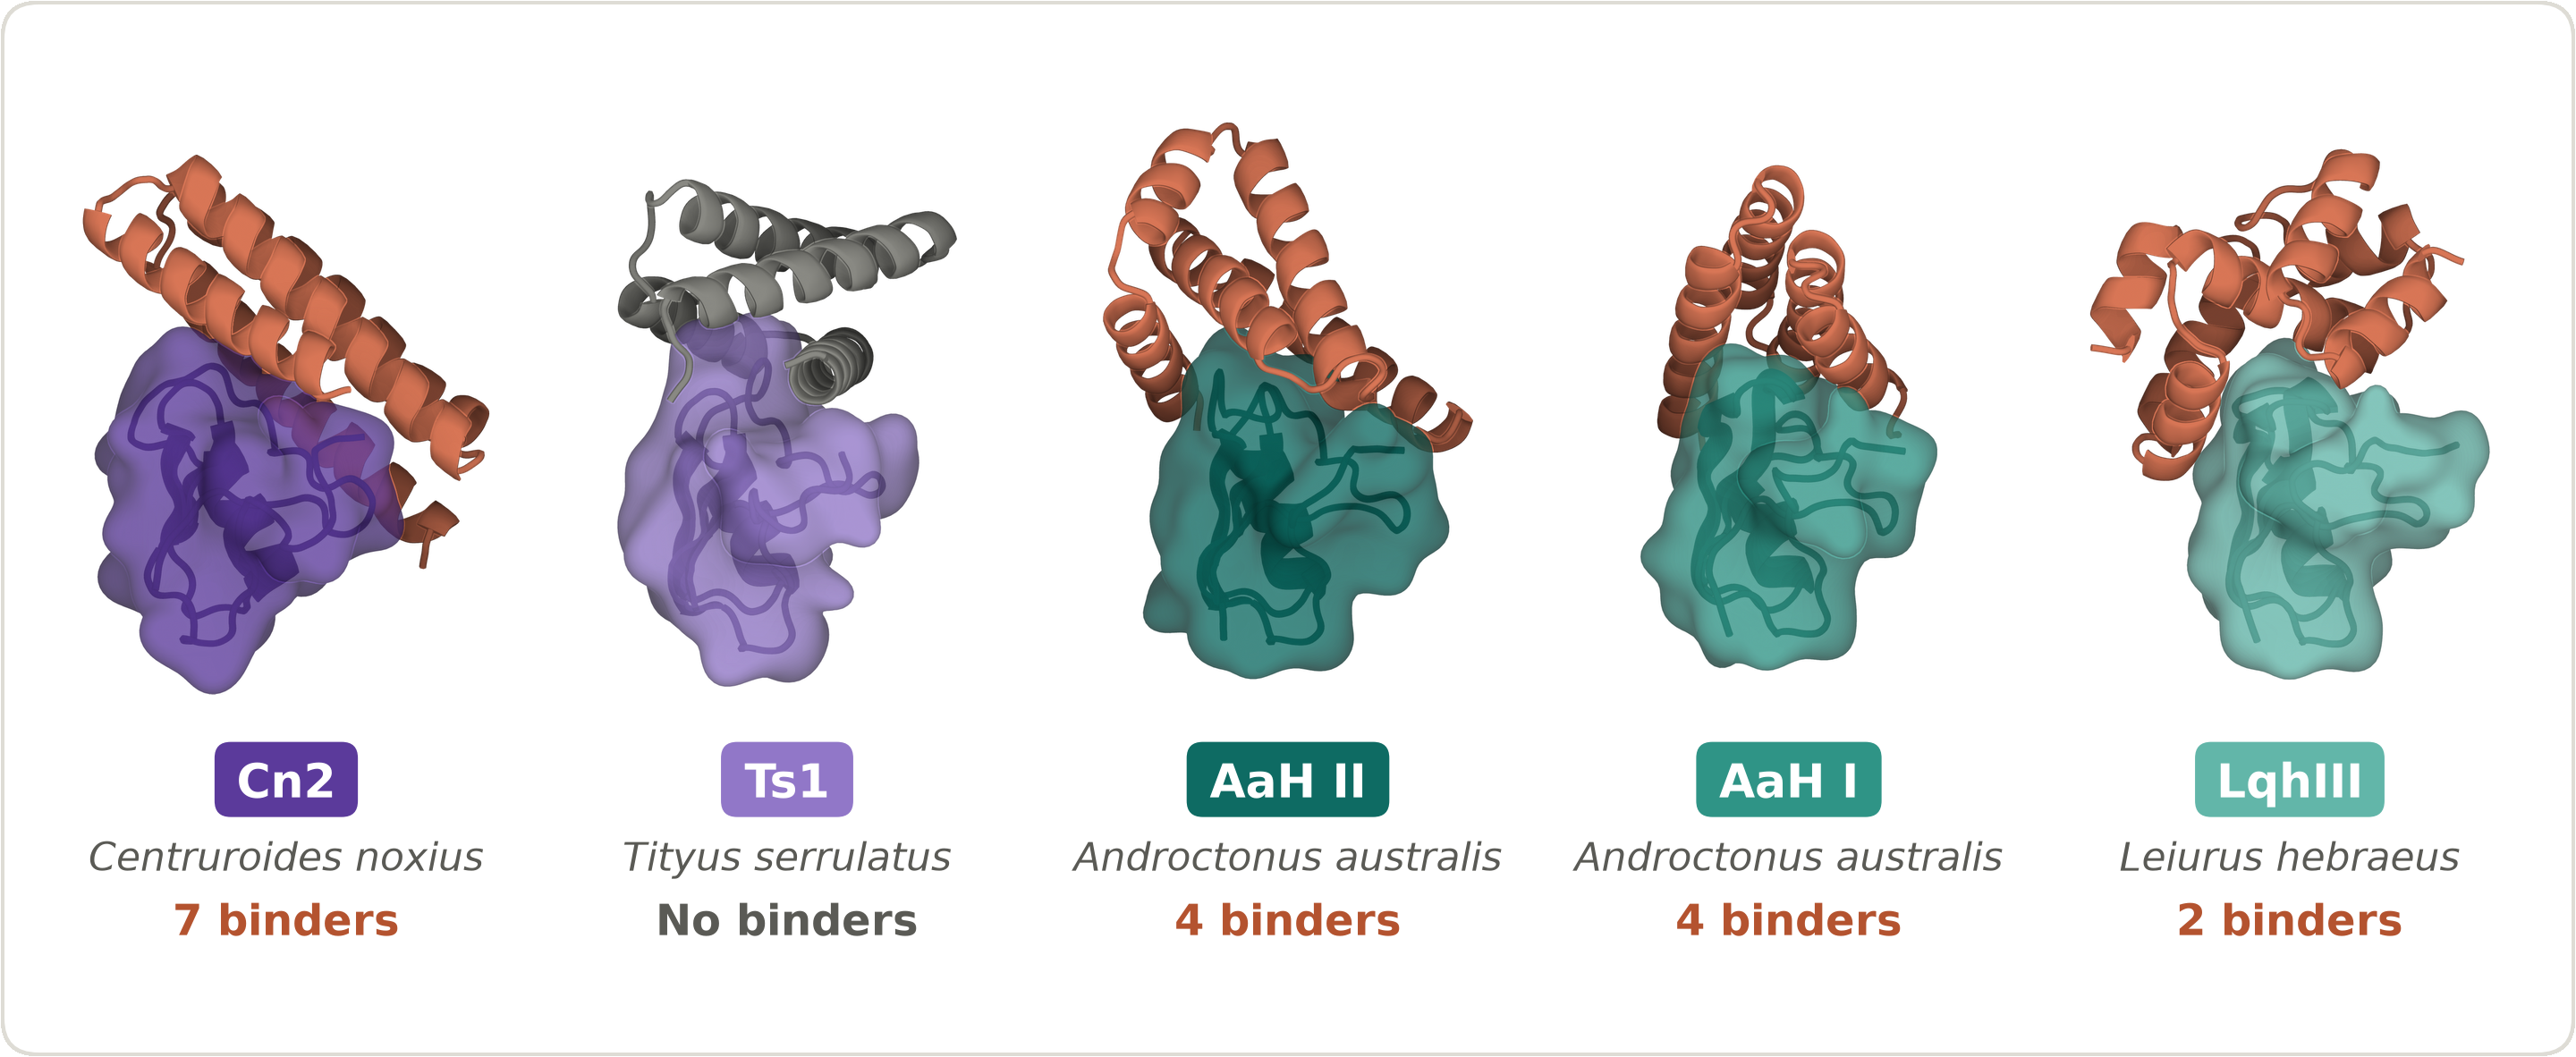
We were primarily wondering if Claude could design binders against individual toxins. But we were also curious if Claude could design binders that targeted multiple toxins. There’s a practical reason for trying to design multitoxin binders, namely that it would reduce the number of molecules needed for a universal antivenom cocktail—which would be the most cost-effective and regionally neutral treatment. We selected these five scorpion toxins (Cn2, Ts1, AaH I, AaH II, and LqhIII) as a challenging test of multitoxin design: they share one fold for the overall shape of the protein, but any two are only 26% to 62% identical in their amino acid sequences.
To see how far Claude could go, we asked it to design four kinds of binders: binders against each of the five toxins individually; binders that targeted the β-family toxins Ts1 and Cn2; binders that targeted the α-family toxins AaH II, AaH I, and LqhIII; and binders that targeted all five toxins simultaneously.
Designing credible binders against five toxins in parallel, in a matter of days, is a great showcase of the AI-driven paradigm shift we are seeing in therapeutic discovery. This is especially true for neglected diseases such as animal envenomings, which have been largely starved of innovation due to low commercial incentives. Being able to agentically tackle the uniquely broad target space across animal toxins provides a significant speed-up in discovery, and brings realistic therapeutic solutions much closer.
Timothy P. Jenkins, Associate Professor, Technical University of Denmark.
Claude ran the design campaign with considerable autonomy
Our initial prompt defined the neurotoxin targets, the protein design and folding tools, and the rules for novelty, scoring, and filtering. Beyond choosing the structures and amino acid hotspots, Claude also set the quality thresholds a design had to clear, decided how much to lean on each available design tool, and developed the strategies for designing binders against multiple toxins.
Ultimately, Claude used 12 design tools to generate 318,484 designs, filtering out any that resembled a toxin or a known protein. Claude co-folded and screened 553,052 design-toxin pairs, predicting each pair’s structure as one complex. Sixty-four hours after we gave Claude our initial prompt, it produced its final list of 180 designs. The campaign used on the order of 10,000 GPU hours.2
Claude worked autonomously for 24 hours following our first prompt. Its results encouraged us to prompt Claude to continue its campaign and look for better designs. Our follow-up prompts were mainly focused on directing Claude to design a multitoxin binder. Claude selected most of the 180 designs—including our strongest binder (Cn2-B1)—only after our third follow-up. At our request, Claude sent the protein sequences to Twist Bioscience (in emails indicating they were written by Claude), which produced the proteins in order to see how well they would bind to the toxins. We later worked with Claude to add another 31 designs, increasing the total to 211 designs: 60 designs against a single toxin (12 per toxin), 30 designs against the two β-family toxins, 30 designs against the three α-family toxins, and 91 designs against all five toxins.
Of the 211 designs our teams assessed, 17 met our criteria for a binder, each against a single toxin. None of the designs made against multiple toxins met our criteria for more than one. (Beyond being limited by its current capabilities, there could be many explanations for why Claude struggled with this, including our prompting, the limitations of available design tools, and even the biological feasibility of multitoxin design.) Seven designs were binders against Cn2, four against AaH II, four against AaH I, and two against LqhIII. Among the 60 single-toxin designs, 11 were binders (18%). This rate is consistent with typical protein design campaigns, including our previous work.
Testing Claude's designs in the lab
After completing the campaign, we sent the designs to Adaptyv Bio and Twist Bioscience to test them for binding. Each group produced the designs in their labs, but in different formats. Adaptyv Bio expressed them in a cell-free system, which uses protein-making machinery extracted from bacteria rather than living cells. Twist Bioscience expressed the designs in mammalian cells (in this case, human kidney cells) as fusions to Fc, the stem of an antibody. These are complementary ways to measure the underlying binding process, and we combined them in order to improve confidence in our results.
Both labs measured binding by surface plasmon resonance (SPR), in which a toxin flows over the design while the SPR instrument tracks in real time how quickly a toxin binds to and detaches from it. The resulting trace, called a sensorgram, produces a measurement known as the dissociation constant (KD), which is a measurement for binding strength (or affinity). The lower the KD, the tighter the binding.
When it came to evaluating the resulting designs, we set out strict criteria for labeling a design a binder against a toxin. The design needed to be a hit at both labs3—that is, it needed to show evidence of binding against that toxin in every replicate, and every KD needed to be 1 µM or tighter. We also required that the design show no signal against CLEC12A, an unrelated human protein used to measure off-target binding or “stickiness.”
Claude’s Cn2 binders likely bind the same site as a toxin-neutralizing antibody
Antibodies and nanobodies remain the standard for de novo designs to beat. Three such molecules have reported affinities (KD) below 1 nM (nanomolar) against Cn2 or AaH II, and they have been shown to protect mice from scorpion toxins.
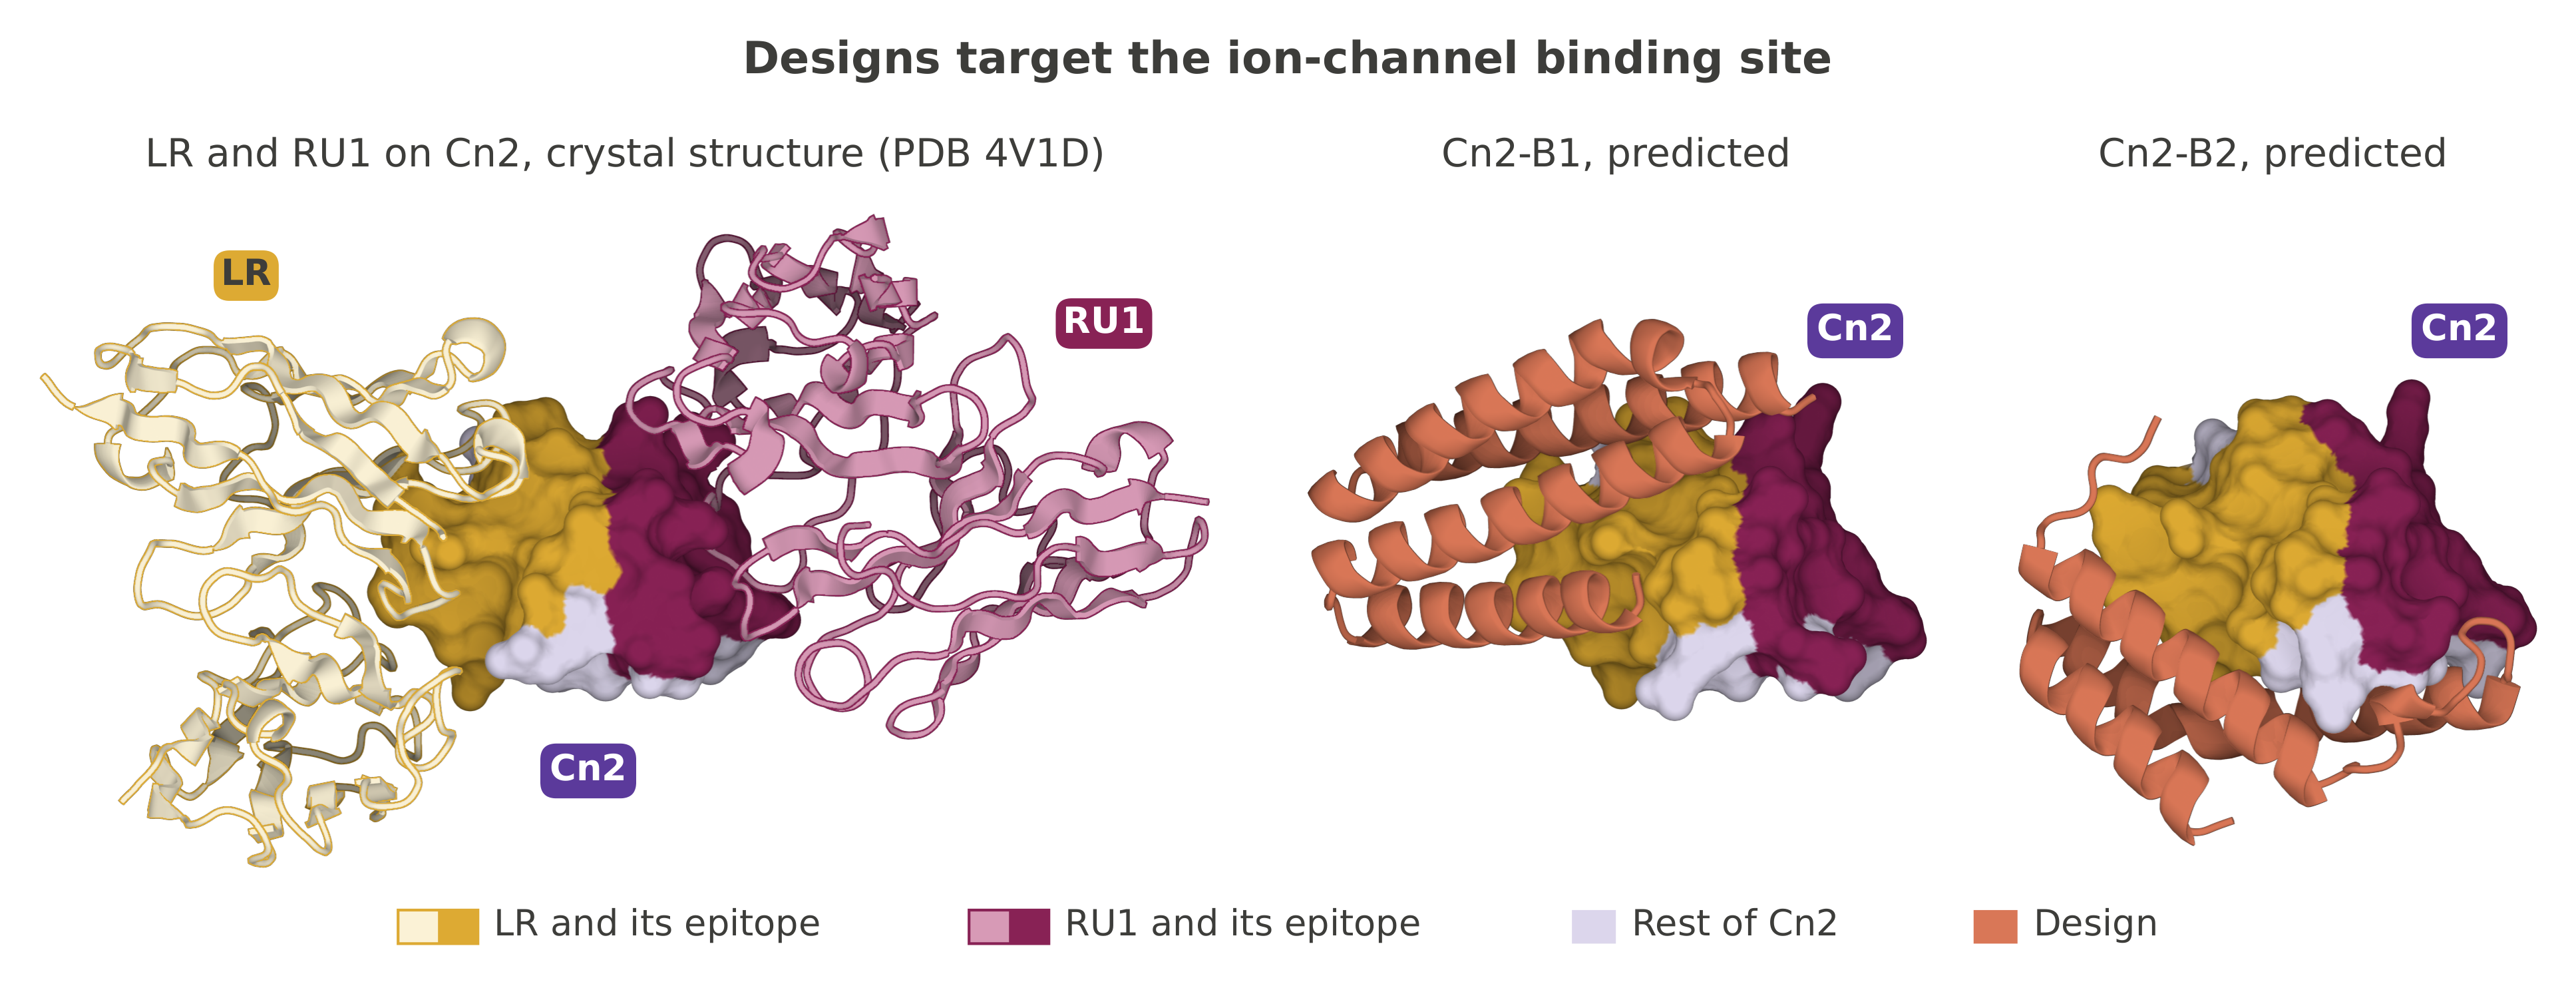
Our two strongest binders, which we call Cn2-B1 and Cn2-B2, target Cn2, a neurotoxin from the Mexican scorpion Centruroides noxius. They each bound Cn2 tightly at both Adaptyv Bio and Twist Bioscience, with affinities (KD) in the single-digit nanomolar range.
One way to find out whether two molecules (e.g., an antibody and a miniprotein) bind the same site on a target is with a competition experiment, which tests whether both binders can attach to the target at the same time. If the presence of one molecule reduces the other molecule’s binding, then they likely compete for the same binding site.
Our competition experiments suggest our Cn2 binders each attach on or near the same epitope (binding site) as an antibody called LR, which has been reported to neutralize Cn2 in mice. LR’s binding site covers the part of Cn2 that attaches to the sodium channel and causes nerves to misfire. We have not tested our strongest binders, Cn2-B1 and Cn2-B2, in a cellular environment or in live animals, but the fact that they compete with LR suggests that they will likely neutralize Cn2.
A binder is only the first step to developing an antivenom
Our results show binding only against recombinant toxins, which are grown in the lab from each toxin’s gene rather than purified from venom. The two biggest limitations of this study are that we didn’t test any design for neutralization in vitro (against cells grown in the lab) or for efficacy in vivo (in living animals, such as mice).
If we were to advance one design toward a therapy, Cn2-B1 would be one of our strongest candidates. First, though, we would need to confirm the design also binds toxin purified from venom. We would then assess it for function in vitro with patch-clamp recordings (which can measure the electrical current passing through sodium channels) to see whether it stops the toxin from acting on the channel. Then, we would need to test the binder in mice to see whether it actually protects them. Beyond neutralizing the toxin, a treatment must also be safe, stable, affordable, and available where stings occur. Reaching patients will also take cooperation from clinicians, funders, and policymakers.
We are releasing all 211 designs and their binding data so that other researchers can build on our work. We hope this demonstration of Claude’s capabilities, along with the data we are releasing, will help accelerate further research into antivenom design.
Further reading
The following resources provide further technical depth and more detailed information about the results described above:
- Technical report;
- Data release: all 211 designs, their predicted structures and scores, and experimental data;
- Our previous posts on protein design and uplifting biomolecular modeling.
Footnotes
01Citrini has written an article on our collaboration, here.
02We realize this is much more than most researchers have access to. Separately, we have made these models about 4x faster on average, and shown that a simplified prompt using a single agent and a single GPU over 24 hours reaches comparable in silico scores.
03LqhIII was assessed only by Adaptyv Bio.